
Description
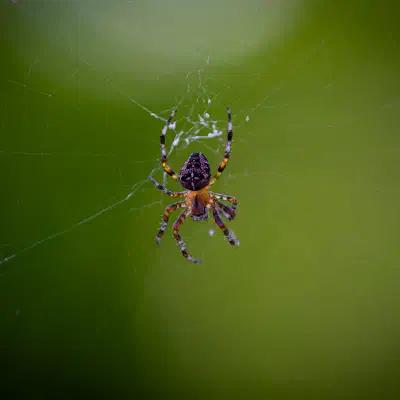
Generally, orb-weaving spiders are three-clawed builders of flat webs with sticky spiral capture silk. The building of a web is an engineering feat, begun when the spider floats a line on the wind to another surface. The spider secures the line and then drops another line from the center, making a “Y”. The rest of the scaffolding follows with many radii of nonsticky silk being constructed before a final spiral of sticky capture silk. The third claw is used to walk on the nonsticky part of the web. Characteristically, the prey insect that blunders into the sticky lines is stunned by a quick bite, and then wrapped in silk. If the prey is a venomous insect, such as a wasp, wrapping may precede biting and/or stinging. Much of the orb-spinning spiders’ success in capturing insects depends on the web not being visible to the prey, with the stickiness of the web increasing the visibility, thus decreasing the chances of capturing prey. This leads to a trade-off between the visibility of the web and the web’s prey-retention ability. Many orb-weavers build a new web each day. Most orb-weavers tend to be active during the evening hours; they hide for most of the day. Generally, towards evening, the spider consumes the old web, rests for about an hour, then spins a new web in the same general location. Thus, the webs of orb-weavers are generally free of the accumulation of detritus common to other species, such as black widow spiders. Some orb-weavers do not build webs at all. Members of the genera Mastophora in the Americas, Cladomelea in Africa, and Ordgarius in Australia produce sticky globules, which contain a pheromone analog. The globule is hung from a silken thread dangled by the spider from its front legs. The pheromone analog attracts male moths of only a few species. These get stuck on the globule and are reeled in to be eaten. Both genera of bolas spiders are highly camouflaged and difficult to locate. In the Araneus diadematus, variables such as wind, web support, temperatures, humidity, and silk supply all proved to be variables in web construction. When studied against the tests of nature, the spiders were able to decide what shape to make their web, how many capture spirals, or the width of their web. Though it could be expected for these spiders to just know these things, it is not well researched yet as to just how the arachnid knows how to change their web design based on their surroundings. Some scientists suggest that it could be through the spider’s spatial learning on their environmental surroundings and the knowing of what will or will not work compared to natural behavioristic rules. The spiny orb-weaving spiders in the genera Gasteracantha and Micrathena look like plant seeds or thorns hanging in their orb-webs. Some species of Gasteracantha have very long, horn-like spines protruding from their abdomens. One feature of the webs of some orb-weavers is the stabilimentum, a crisscross band of silk through the center of the web. It is found in several genera, but Argiope – the yellow and banded garden spiders of North America – is a prime example. As orb-weavers age, they tend to have less production of their silk; many adult orb-weavers can then depend on their coloration to attract more of their prey. The band may be a lure for prey, a marker to warn birds away from the web, and a camouflage for the spider when it sits in the web. The stabilimentum may decrease the visibility of the silk to insects, thus making it harder for prey to avoid the web. The orb-web consists of a frame and supporting radii overlaid with a sticky capture spiral, and the silks used by orb-weaver spiders have exceptional mechanical properties to withstand the impact of flying prey. The orb-weaving spider Zygiella x-notata produces a unique orb-web with a characteristic missing sector, similar to other species of the Zygiella genus in the Araneidae family. During the Cretaceous, a radiation of flowering plants and their insect pollinators occurred. Fossil evidence shows that the orb web was in existence at this time, which permitted a concurrent radiation of the spider predators along with their insect prey. The capacity of orb–webs to absorb the impact of flying prey led orbicularian spiders to become the dominant predators of aerial insects in many ecosystems. Insects and spiders have comparable rates of diversification, suggesting they co-radiated, and the peak of this radiation occurred 100 Mya, before the origin of angiosperms. Vollrath and Selden (2007) make the bold proposition that insect evolution was driven less by flowering plants than by spider predation – particularly through orb webs – as a major selective force. On the other hand some analyses have yielded estimates as high as 265 Mya, with a large number (including Dimitrov et al 2016) intermediate between the two. Most arachnid webs are vertical and the spiders usually hang with their heads downward. A few webs, such as those of orb-weavers in the genus Metepeira, have the orb hidden within a tangled space of web. Some Metepiera species are semisocial and live in communal webs. In Mexico, such communal webs have been cut out of trees or bushes and used for living fly paper. In 2009, workers at a Baltimore wastewater treatment plant called for help to deal with over 100 million orb-weaver spiders, living in a community that managed to spin a phenomenal web that covered some 4 acres of a building, with spider densities in some areas reaching 35,176 spiders per cubic meter.